A soil test measures nitrogen in solution and on exchange sites at the moment you sampled. It does not measure the nitrogen already inside living microbial cells. That single omission is the most common reason a nitrogen result reads lower than the fertiliser record says it should. Nitrogen immobilization is the process behind it. A large share of the nitrogen that appears to vanish after residue incorporation has not left the field at all, because nitrogen immobilization has moved it into microbial biomass, where no extraction method used in routine testing will find it, and where it stays until something eats the microbe holding it.
What a routine soil test can and cannot see
Standard mineral nitrogen tests extract ammonium and nitrate from the soil solution and from cation exchange sites. This is the pool a root competes for, so measuring it is reasonable.
The limitation is what falls outside the extraction. Nitrogen held in microbial biomass sits inside intact cells. It is not extracted, so it is not reported. Total soil nitrogen has not changed, but the number on your report has, and nitrogen immobilization is the reason for the difference.
The practical result is that immobilized nitrogen and leached nitrogen look identical on a soil test. One is recoverable within weeks. The other is gone for the season. The test cannot tell you which one you are looking at, which is why reading a low result without knowing the residue history of the field is guesswork.
Why decomposers pull nitrogen out of the soil solution
Microbes decomposing plant residue are working with a carbon source. Building new cells from that carbon requires nitrogen, because proteins, nucleic acids and cell wall components all contain it.
When the residue supplies plenty of carbon and very little nitrogen, decomposers are limited by nitrogen rather than by energy. They take the shortfall from wherever it is available, which is the mineral nitrogen already in the soil solution. That is the same ammonium and nitrate a root would otherwise have taken up.
This is net nitrogen immobilization. It is not a malfunction, and it is not competition in any adversarial sense. It is stoichiometry, and it happens in every soil where fresh carbon arrives faster than nitrogen does. A cell cannot be built out of carbon alone.
The 25 to 1 threshold that triggers nitrogen immobilization
The rule of thumb is that residue with a carbon to nitrogen ratio above roughly 25 to 1 causes net nitrogen immobilization, and residue below it causes net mineralization.
That threshold is derived rather than measured. It comes from two properties of the decomposer community. The first is biomass stoichiometry: bacterial biomass runs at a carbon to nitrogen ratio near 5 to 1, fungal biomass considerably wider, and a mixed community somewhere near 8 to 1. The second is carbon use efficiency, the fraction of consumed carbon retained as biomass rather than respired, typically around 0.3 for a mixed soil community.
Divide community stoichiometry by carbon use efficiency and you arrive near 25. This is why the nitrogen immobilization threshold shifts with residue quality, temperature and community composition rather than holding as a fixed constant across every field.
For context, cereal straw commonly runs between 80 and 100 to 1, which puts it well inside immobilizing territory. Legume residue runs closer to 15 to 20 to 1. Compost that has already been through a decomposition cycle usually sits below the threshold, which is one reason it behaves so differently from fresh residue carrying the same total nitrogen content.
Nitrogen immobilization is a delay, not a loss
The important consequence of the mechanism is directional. Leached nitrate has moved below the root zone and is not coming back this season. Volatilized ammonia is in the atmosphere. Nitrogen immobilization leaves the nitrogen thirty centimetres from where you applied it, inside a cell, still inside the field boundary.
Studies using labelled nitrogen consistently recover a substantial fraction of applied fertiliser in the soil organic and microbial pool within the first weeks after application. The reported ranges vary widely with soil type, residue quality and placement, so the figure is worth checking against a study matched to your own conditions rather than quoting a single number as though it were universal.
What matters agronomically is that nitrogen immobilization has a return path. The other loss routes do not.
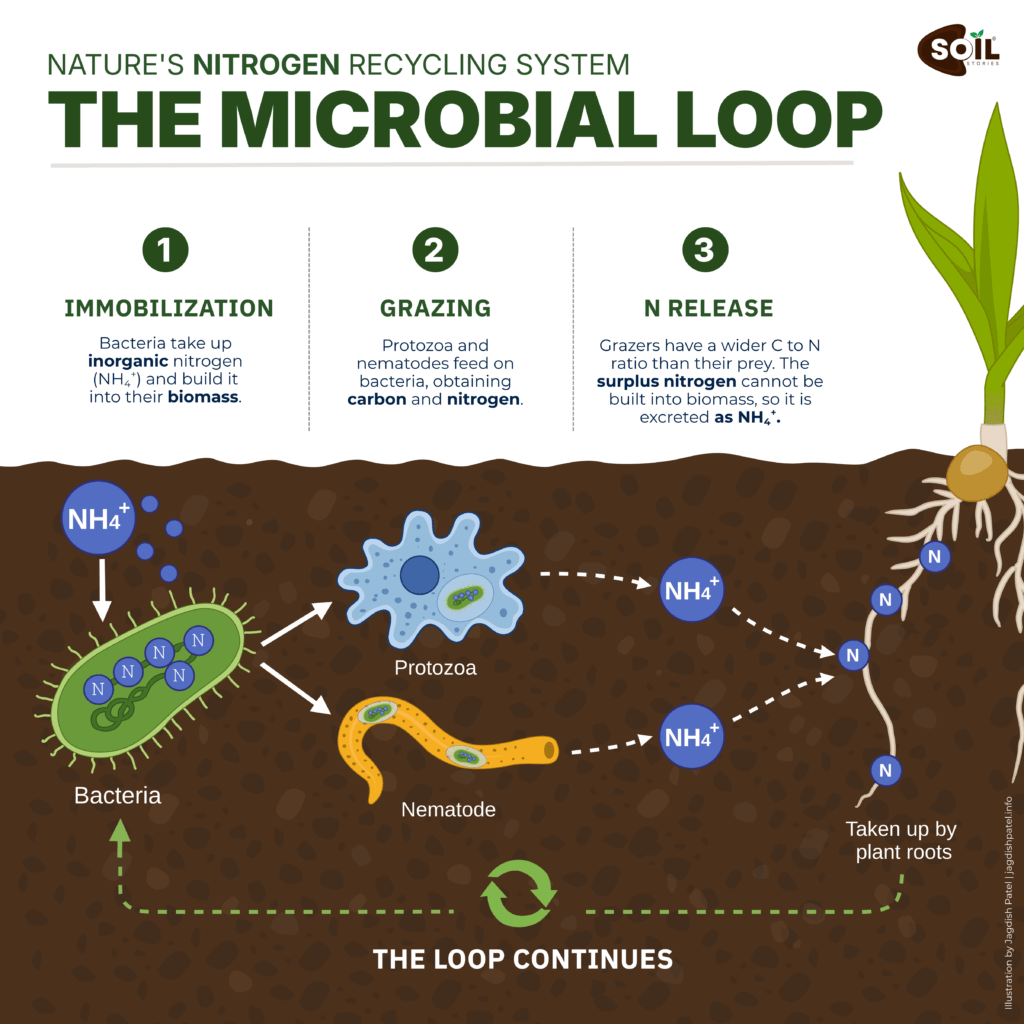
How the nitrogen comes back: The soil microbial loop
Microbes do not release nitrogen because they have finished with it. A living bacterium holds its nitrogen indefinitely, and a large share of the soil bacterial population is dormant rather than actively turning over. Reversing nitrogen immobilization therefore depends on something other than time.
It depends on predation.
Bacterivorous protozoa and nematodes eat bacteria and take in bacterial carbon and bacterial nitrogen together, in whatever ratio the prey cell held them. The grazer has a wider carbon to nitrogen ratio in its own biomass than its prey, and its carbon use efficiency is lower. It needs more carbon per unit of nitrogen than a bacterial cell actually contains.
The consequence is unavoidable. Nitrogen taken in beyond the grazer’s structural requirement cannot be built into grazer biomass, so it is excreted. It leaves as ammonium.
This is the soil microbial loop, described by Marianne Clarholm in 1985 and refined by later work on protozoan contributions to plant nitrogen supply. Nitrogen becomes plant available because something eats the organism holding it. Grazing is the release valve on nitrogen immobilization.
Why the release happens where the root can use it
The location of the release is not incidental.
Bacterial density is highest in the rhizosphere, because root exudates supply the carbon that supports it. Protozoa and nematodes concentrate where their prey concentrates, which puts grazer activity in the same zone. Ammonium excreted by a grazer is released inside the volume of soil the root is already exploring.
Under aerobic conditions a proportion nitrifies to nitrate before uptake. Roots take up both forms, so the distinction affects mobility and loss risk rather than availability itself.
This spatial coupling is why microbially mediated nitrogen supply is often better synchronised with crop demand than a single broadcast application. The release follows root activity, because root activity is what feeds the bacteria that drove nitrogen immobilization in the first place.
What nitrogen immobilization changes about nitrogen management
Three practical consequences follow from the mechanism.
Residue carbon to nitrogen ratio belongs in the rate decision. A field with heavy cereal residue incorporated at planting carries a different early season nitrogen demand from a field following a legume, even at an identical soil test value, because the nitrogen immobilization potential of the two situations is not comparable.
Placement matters whenever residue is present. Nitrogen banded away from a residue rich surface layer meets fewer decomposers than nitrogen broadcast directly onto it.
Timing beats total rate under immobilizing conditions. Splitting applications reduces the quantity of mineral nitrogen exposed to nitrogen immobilization during the peak decomposition phase, when decomposer demand is highest and crop demand is often still low.
The misconception worth correcting
Microbial biomass is frequently described in agricultural marketing as a nitrogen source. It is a nitrogen sink that becomes a source only when it is grazed.
The distinction is not academic. A soil with high microbial biomass and a depressed grazer population will hold nitrogen rather than supply it, and nitrogen immobilization in that soil looks permanent even though it is not. Biomass measurements alone say nothing about the rate of return. That rate is governed by the food web above the bacteria, not by the size of the bacterial pool.
Nitrogen management built on the assumption that feeding soil biology automatically increases availability has the mechanism half right. Feeding biology builds the pool. Predation empties it.
Frequently asked questions about nitrogen immobilization
Does immobilized nitrogen become available again?
Yes. Nitrogen immobilization is reversible. The nitrogen returns to the soil solution mainly through predation of bacteria by protozoa and nematodes, which excrete surplus nitrogen as ammonium.
What carbon to nitrogen ratio causes nitrogen immobilization?
Residue above roughly 25 to 1 generally causes net nitrogen immobilization. Cereal straw commonly falls between 80 and 100 to 1, and legume residue closer to 15 to 20 to 1.
Why does a soil test show low nitrogen after adding straw?
Decomposers take mineral nitrogen from the soil solution to process the carbon in the straw. The nitrogen moves into microbial biomass, which routine soil tests do not extract, so nitrogen immobilization reads on the report as a loss.
Sources
Clarholm, M. (1985). Interactions of bacteria, protozoa and plants leading to mineralization of soil nitrogen. Soil Biology and Biochemistry, 17(2), 181-187.
Bonkowski, M. (2004). Protozoa and plant growth: the microbial loop in soil revisited. New Phytologist, 162(3), 617-631.
Recous, S., Robin, D., Darwis, D., Mary, B. (1995). Soil inorganic N availability: effect on maize residue decomposition. Soil Biology and Biochemistry, 27, 1529-1538.
This is the same clarity I bring to brands.
I’m a soil scientist who turned into a visual science communicator. If this article made a hard concept click, that’s exactly what I build for agriculture and AgTech brands: scientific illustrations, infographics, explainer videos, and content that turns complex research into something your customers actually understand and trust.